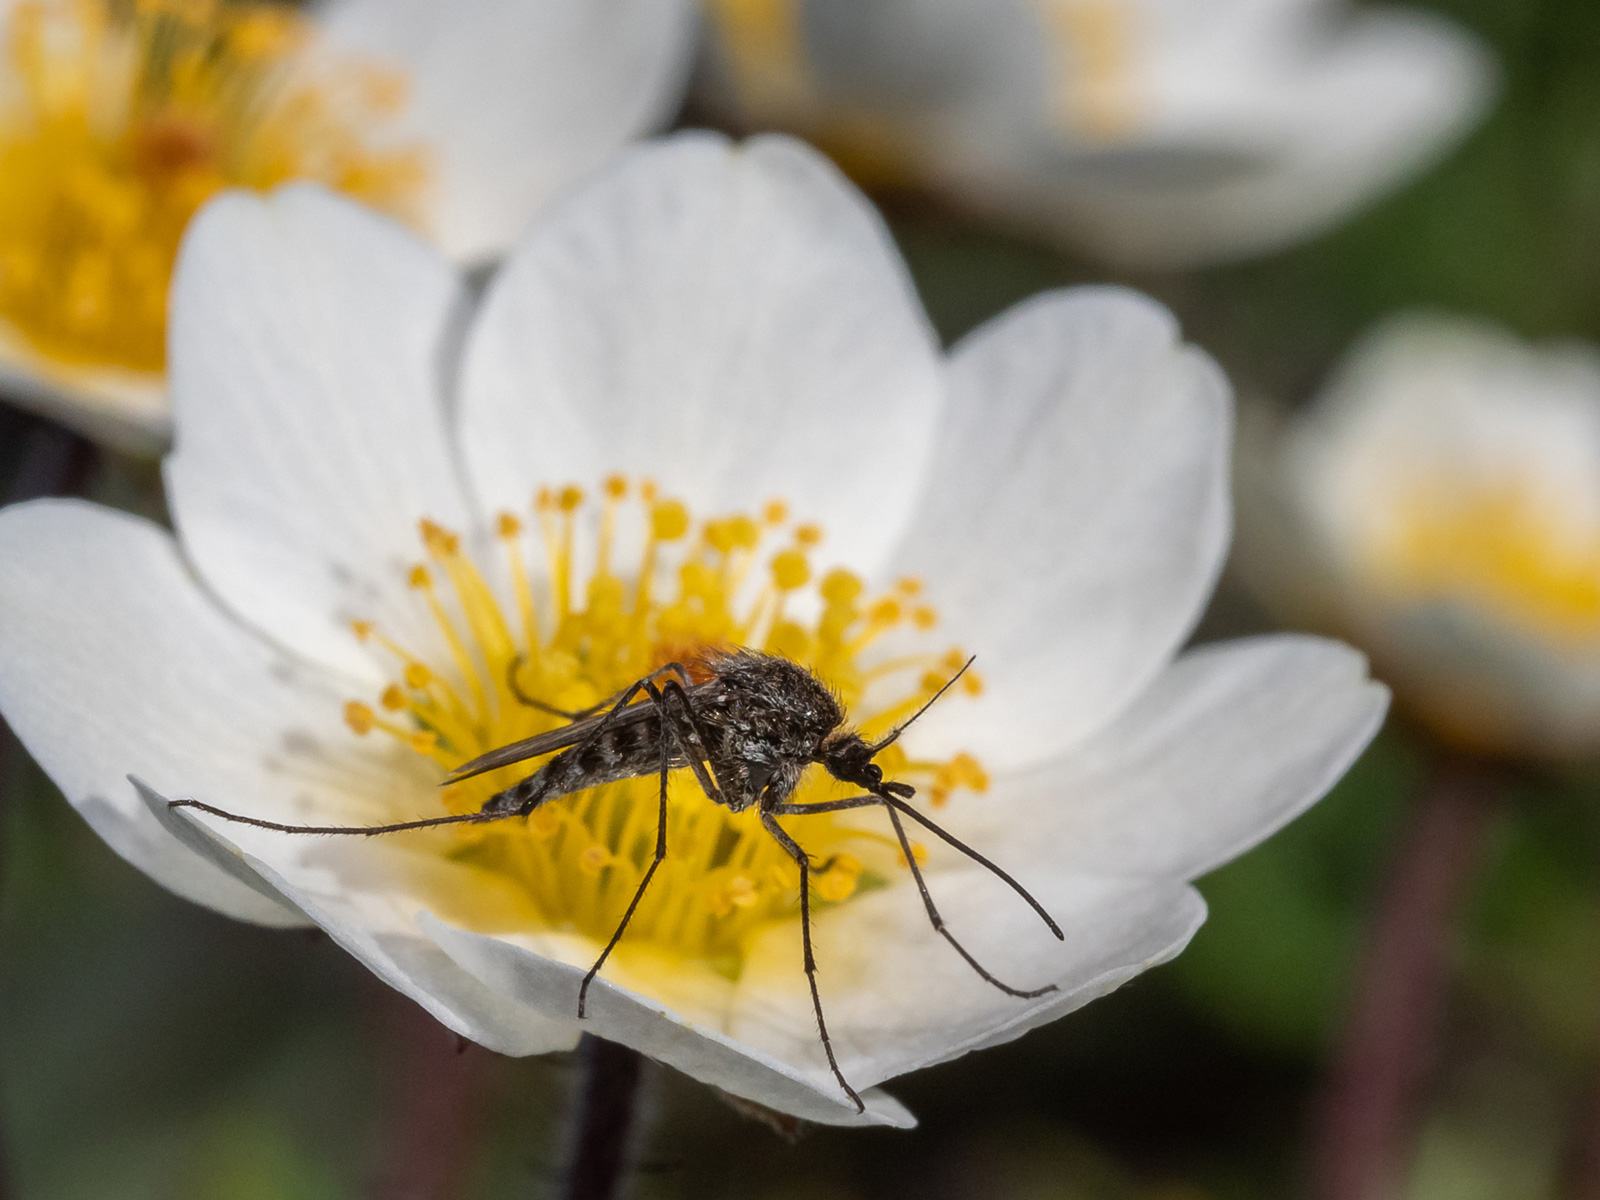
Photo by Piotr Lukasik, some rights reserved (CC BY).
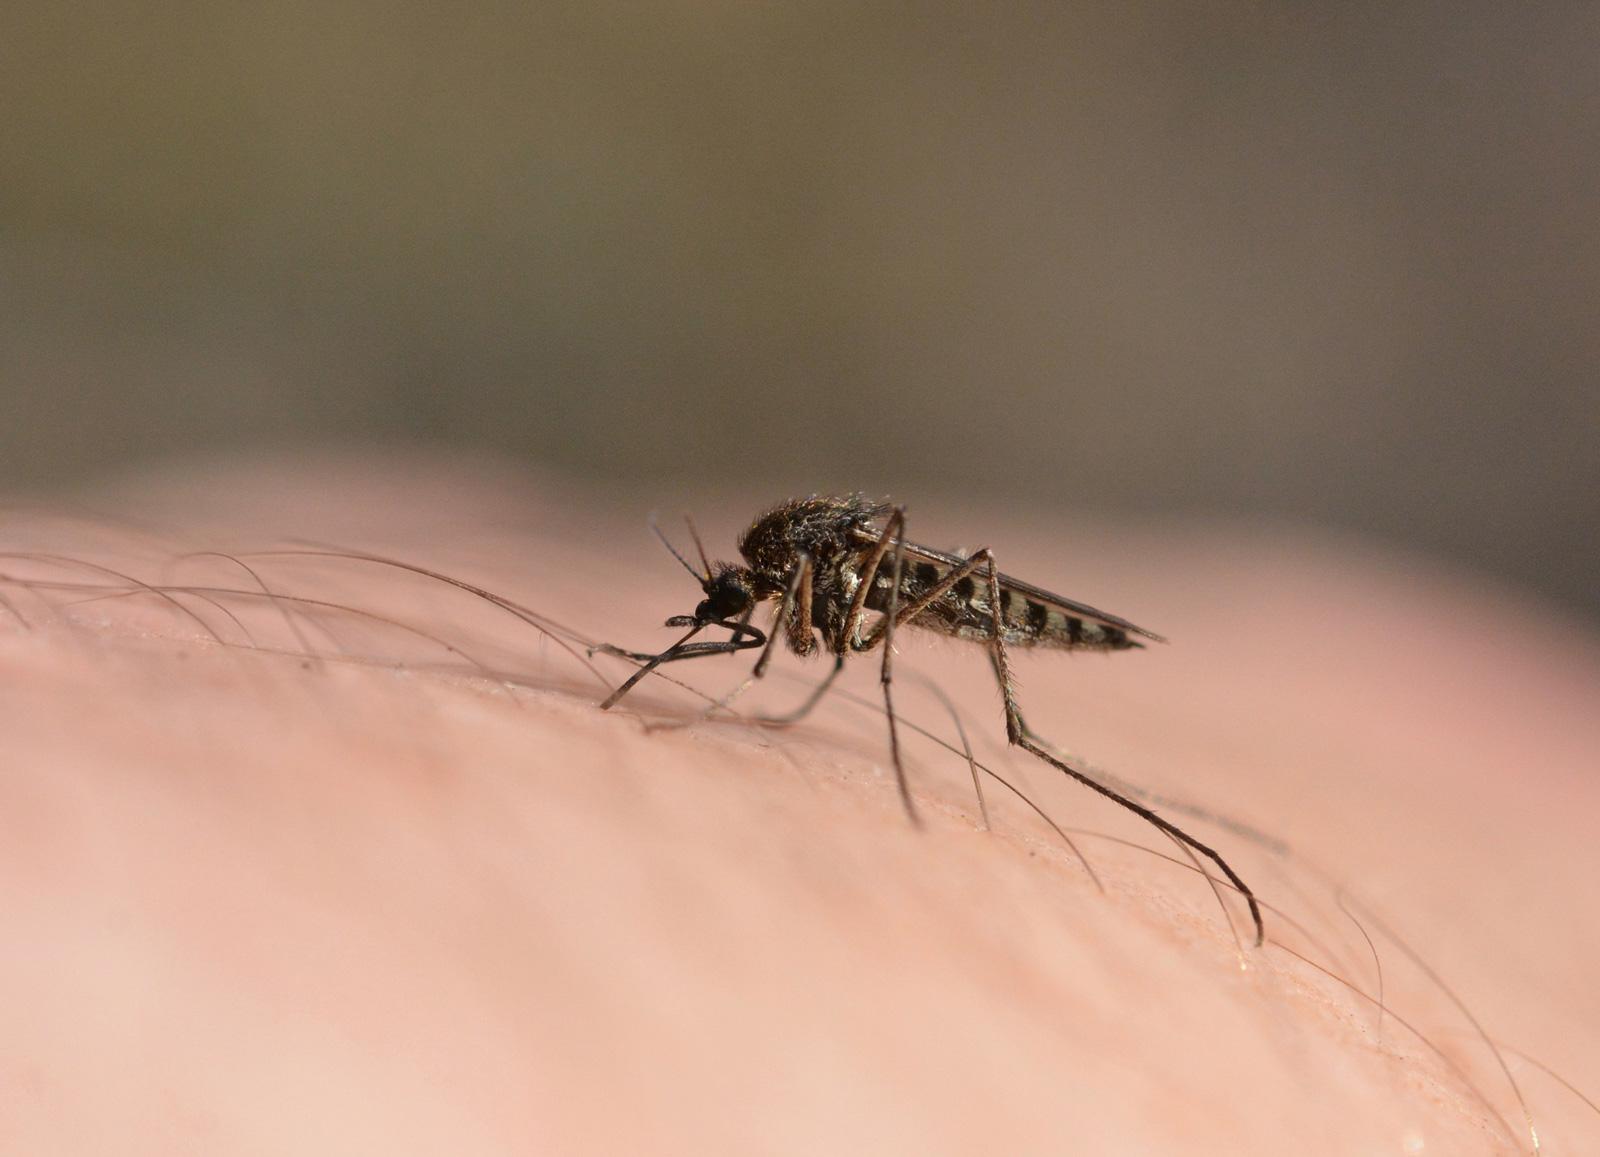
Photo by Anthony B. Zerafa, some rights reserved (CC BY-NC).
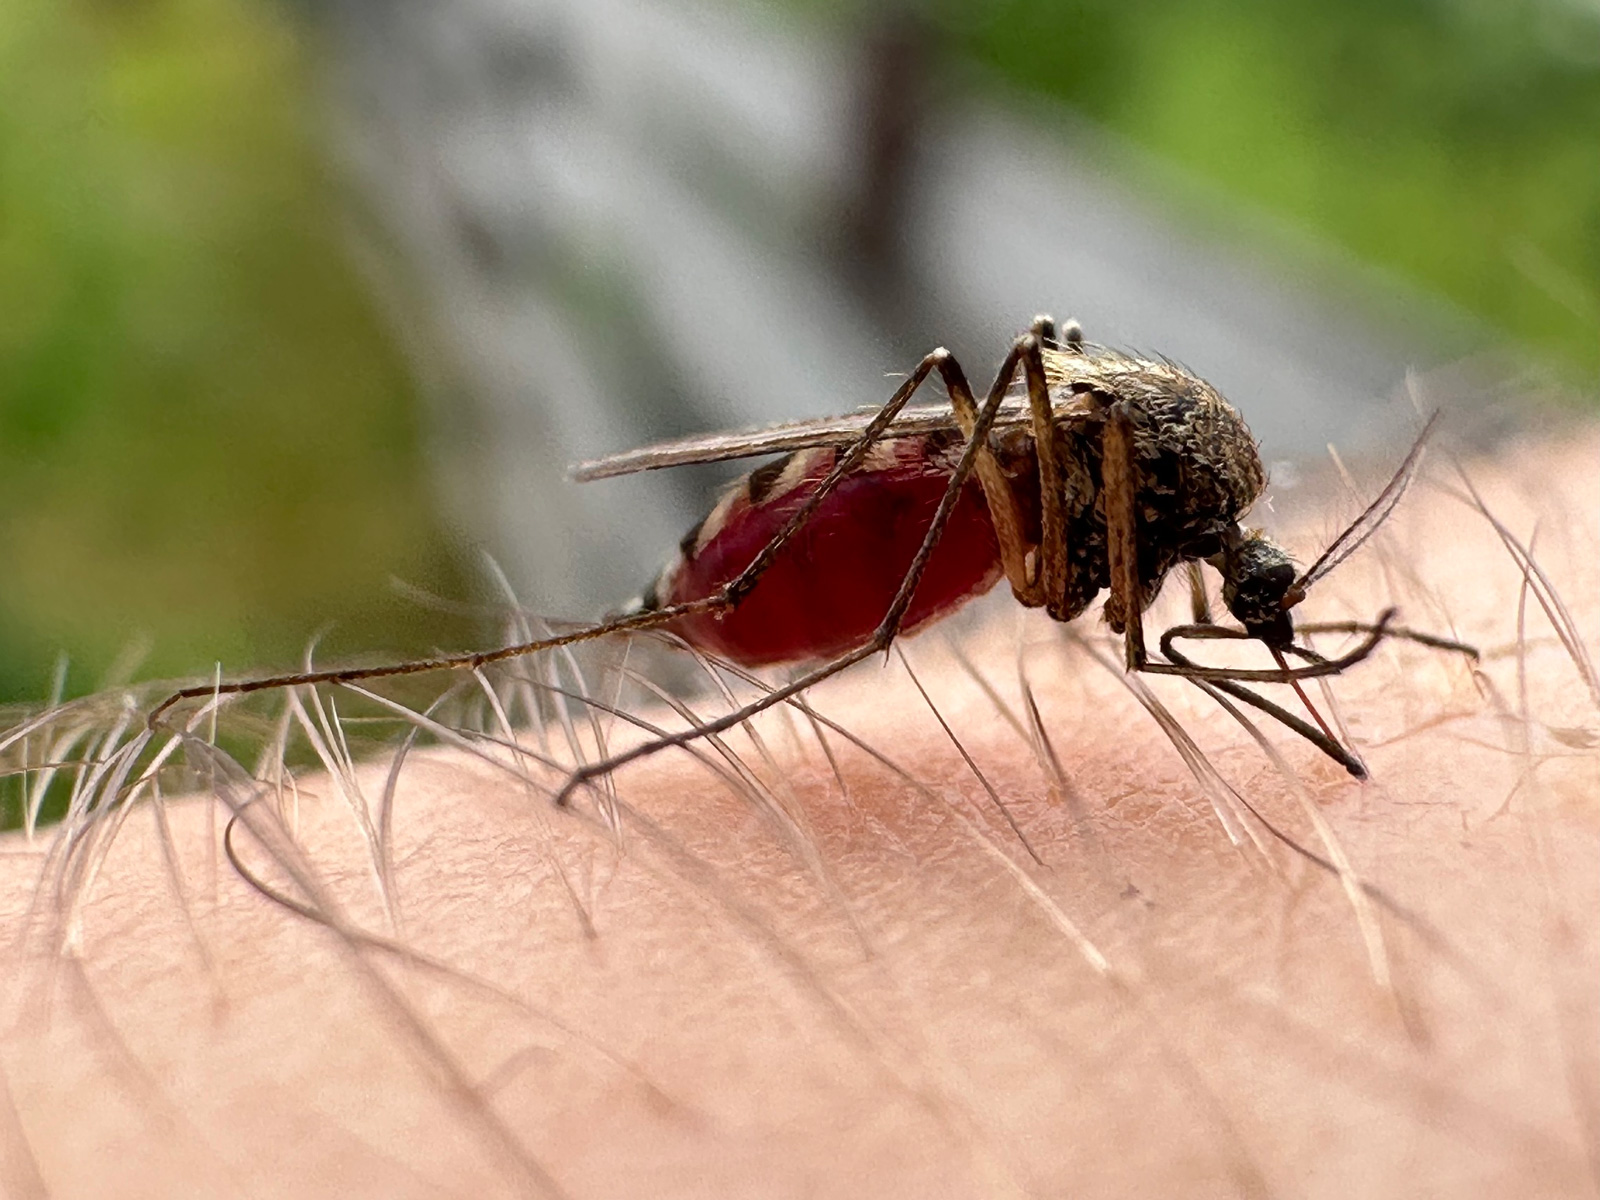
Photo by Stepan Markin, some rights reserved (CC BY-NC).
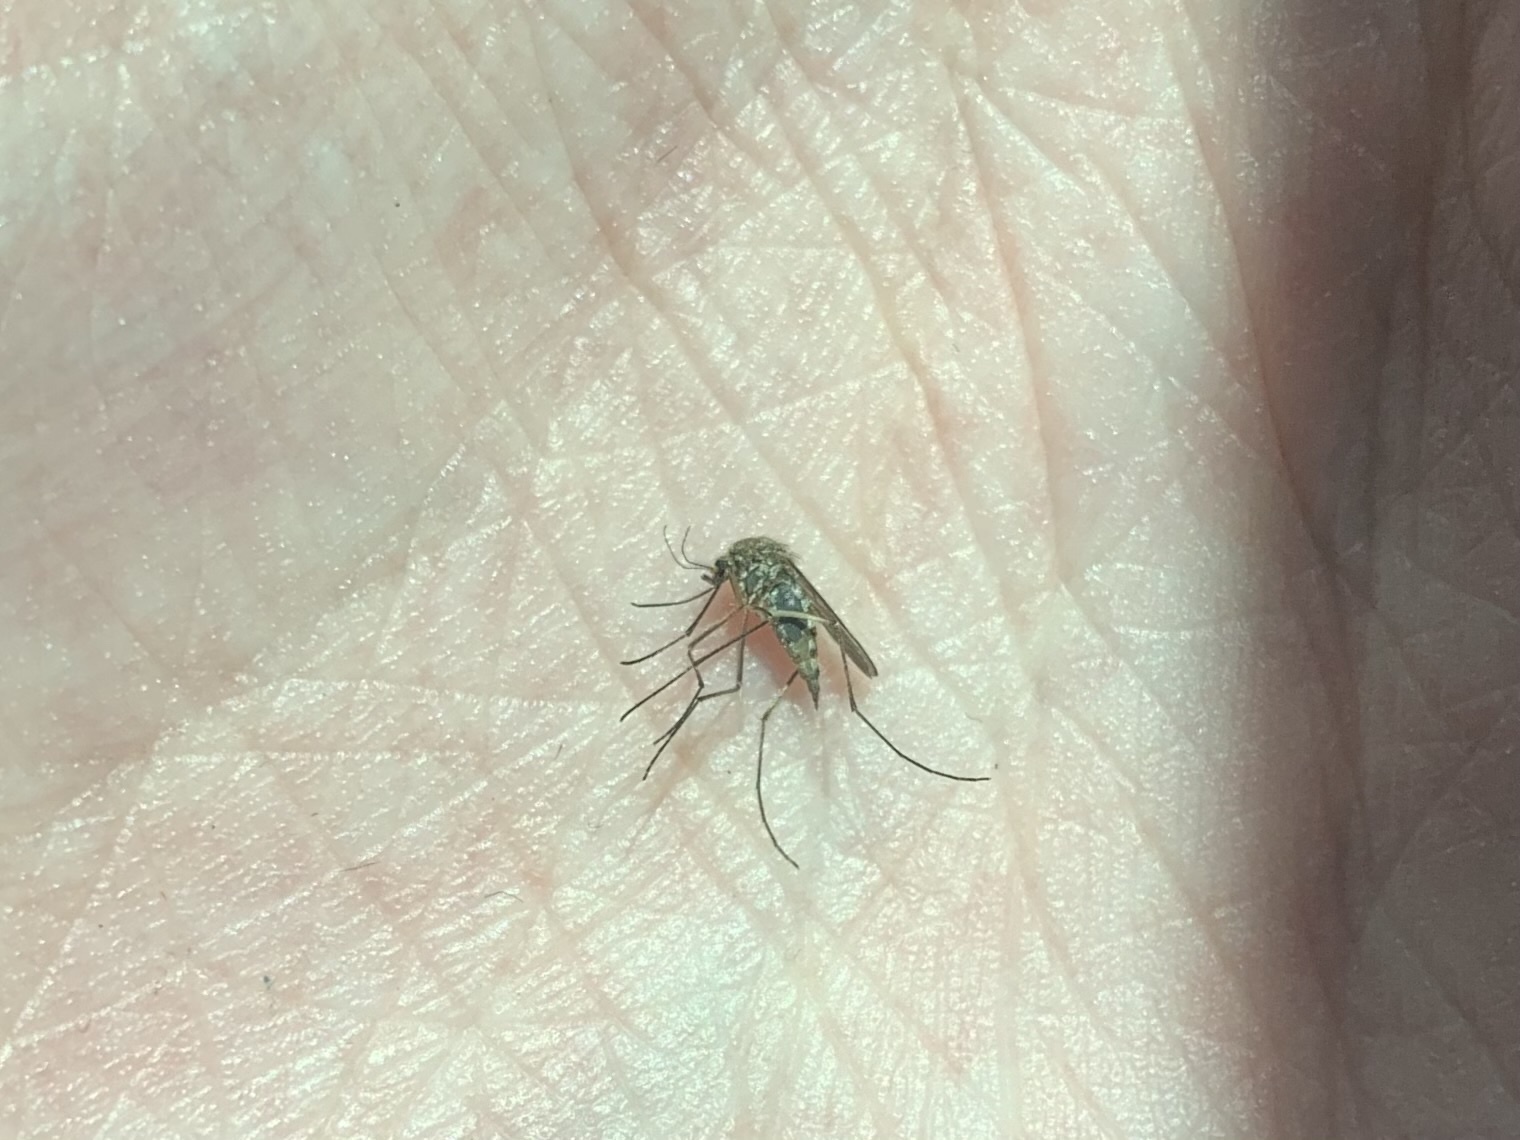
Photo by Lane Keller, some rights reserved (CC BY-NC).
Hairy Tundra: Aedes impiger. Arctic Black-Footed: Aedes nigripes.
Not assessed by the IUCN.
Hairy Tundra: 978 million base pairs. Arctic Black-Footed: 978 million base pairs.
Mosquitoes may be considered to be semi-aquatic animals, or semi-terrestrial, depending on your point of view. Certainly, for the vast majority of the time that an individual is alive and survives to adulthood, the mosquito is an aquatic animal. For Arctic mosquitoes like A. impiger and A. negripes, freshly fertilized eggs are deposited in freshwater bodies (of which there are many in the Arctic tundra (e.g., thermokarsts)), which may be short-lived (ephemeral or vernal (formed by snow melt in the springtime)) or semi-permanent or permanent. After hatching, the first larval stage immediately begins feeding on biofilms (thin mats of bacteria) that coast the substrate in Arctic pools. As the larvae develop further, they feed on increasingly larger elements of pool biota, such as zooplankton, rotifers, and other arthropod larvae. At the same time, they provide an important source of nutrition for the invertebrate biota of Arctic thermokarsts (e.g., predatory diving beetles such as Dytiscids (= Tulugarnaq in Inuktitut)). Once the larvae reach their final pre-adult stage (stages are called ‘instars’), like all metamorphic insects, they pupate for a period – in which they cocoon themselves whilst major anatomical reconstruction is undergone – before emerging as fully functional, airborne and newly terrestrial adults. Interestingly, as the Arctic warms, mosquitoes are increasing the rate at which they develop as a means of predator avoidance. Adult mosquitoes tend to be hematophagous (‘blood eaters’), as most of us can testify. As females are the only adults to feed, hematophagy has been associated with reproductive status. Producing eggs is energy intensive and the short window from converting a liquid meal into eggs that are subsequently laid after coupling with a male (who does not feed as an adult), gives mosquitoes an edge when it comes to reproduction. Adults will feed on large Arctic mammals, as well as incubating waterfowl. However, some species – as has been documented in Aedes negripes – may display autogeny, which means that the females do not feed on blood as a prerequisite for producing a brood of eggs. Autogeny is a highly advantageous trait where the host target species for hematophagous insects are relatively rare (most Arctic terrestrial mammals are widely distributed and less abundant the further north one travels), thus gravid females, once emerged, can put all of their energy stores into finding a mate and maturing eggs to seed the next generation. Eggs mature and are ready for oviposition around 10 days after emergence in both Aedes nigripes and Aedes impiger. However, not depending on blood for energy may come at the cost of maturing a limited number of eggs. Like in a lot of animal behaviour (ethology), there are trade-offs and different strategies to maximise reproductive potential. Eggs are laid in the soil of the tundra during summer around 20mm above the water line of ponds, usually at sites that fill further upon the first thaw of the snowpack the following spring. Eggs are also deposited on south-facing edges, to maximise their exposure to the sun. Here the eggs overwinter in an arrested state of development until the inundation of the ponds the following year.
A component of the qupirruit (insects and worms), qikturiaq, in an everyday sense, are considered a nuisance of the brief Arctic summer, causing airborne mischief whilst the harvesters track their prey and the community go about their business. Close to the treeline, both A. impiger and A. negripes tend to be more active during the solar high during the daytime. As qikturiaq activity increases, so does the risk of Inuit feeling ‘quinak’, a ticklish feeling of extreme annoyance on the skin that comes from alighting and feeding insects.
A paper entitled “Qupirruit: Insects and Worms in Inuit Traditions” by Laugrand and Oosten (2010) conveys some of the Inuit lore surrounding mosquitoes. Qikturiag, according to Inuit legend, are derived from the body of a giant. Quoting from an anonymous source, Laugrand and Oosten report: “A young man went into caves where the giants lived. The Inuk shot a giant in the heel. He fell and became smaller and smaller until he was the same size as the Inuk. The young man went out to inform people who flocked towards the cave. Then they saw the body of the giant was on fire. "All the Inuit looked at the fire; then they looked at the sun. There, flying up from the fire, were thousands and thousands of mosquitoes. The giant, as he burned, was being changed into mosquitoes.” Other Inuit legends tell that mosquitoes originated as particles of dirt flung from a garment, or from the transmogrification of lice! Despite their status of pests, many Inuit insist that mosquitoes be respected, sometimes believing that if not esteemed, this would lead to injurious changes to the weather. In other regions (e.g., Iglulik), mosquito clouds are afforded predictive value, indicating the arrival of bearded seals or herds of caribou. In the dreamworld, mosquitoes may also be portents of death.
To the mind of many people, attempting to rationalize the conservation of mosquitoes would seem to be a perplexing proposition; after all, who would be in favour of critters for whom we present a meal opportunity? However, there are a number of ways in which mosquitoes generally, and A. impiger and A. negripes, in particular, are of conservation interest. Mosquitoes are part of the millions of species of insects that call Earth their home. Insects are thus an essential component of Earth’s biodiversity, providing ecosystem services (e.g., think how much honey that bees make, or how much decomposition fly and beetle larvae process), food for other animals, and aesthetic pleasure in their just being alive (e.g., butterflies). However, anthropogenic climate change has, across all Orders and Families, within the class of Insecta, not been kind as has been reported over the past few years. In 2021, the alarm bell that was rung previously in 2018 for an “insect apocalypse” was given further credence by a slew of papers citing a general decline in insect numbers and biomass, coinciding with damaging human activities, including indirect effects of climate change. However, in the Arctic terrestrial biome, things may be more complicated due to the greater impact that global warming has here compared to the rest of the globe (air temperatures are increasing at 4x the rate elsewhere). This means that some taxa are increasing in abundance. As the permafrost melts, and the number and volume of ephemeral, semi-permanent and permanent pools increase, so does the available habitat for endogenous mosquitoes – and for northerly migrating species. The federal government of Canada monitors the distribution of mosquito species (Explore the data: Mosquito-borne disease surveillance dashboard in Canada — Canada.ca) – and their parasites and pathogens, and the major fear is that disease-carrying species may expand their range north and supplant native species (which, until recently, bore little public health concerns) with disease-carrying species. Monitoring for populations of tiny and hard to identify mosquitoes can be laborious and slow using conventional tools of the trade – anatomical keys and microscopes. That was, however, until researchers started to delve into the DNA. Time for some genomic insights!
Both of our species of focus do not yet have fully sequenced genomes, although they are on the list of species to be processed during the lifespan of the Canada BioGenome Project, however some interesting genetic work has been conducted on that may have real-world applications. Much of this work that has real value to the Arctic tundra biome and for the residents there, involves the mass screening of individuals of mosquito to determine one of two major goals: 1) Identify species distribution trends over time; and 2) to identify novel pathogens and to monitor the prevalence of known parasites and pathogens that cause disease and distress.
The key genetic concept, using informative bits of genomes called ‘DNA barcodes’, was developed here in Canada, published in a paper in 2003 by Paul Herbert and colleagues at the University of Guelph, Ontario. Put simply, key, standardised regions of the genomes of animals, plants and fungi were sequenced to identify the DNA sequence differences between species in these particular genomic regions of interest. By choosing different regions of the genome, a list of suitable genomic regions was identified that yielded for each species, a unique sequence identifier (sequence of DNA letters, A, C, G or T) that is analogous to the unique device identifier (UDI) barcode one can see on products on the shelves of shops. Whilst commercial barcodes are visualised as black and white bars, the genetic ones have a different colour for each of the four variable DNA letters in the DNA barcode sequence. The first region identified that could differentiate between animal species on the basis of their DNA sequences was a region of the mitochondrial genome involved in the biochemistry of respiration, called cytochrome oxidase subunit 1 (or COI for short). In the 20 or so years since, whole genome sequencing has open up the investigation into suitable barcode regions for the easy identification of biological specimens from a sample of the individual itself, without relying on physical identification! That means, if we were to lay a large malaise trap in the Arctic tundra – a trap that specifically targets a broad suite of arthropod targets – then we no longer need to sift through each individual and assign it to species-level using hugely laborious and time-consuming methods. Instead, we can mush the insects together and extract their combined DNA (called total DNA). Because each species can be identified by a barcode sequence, if we apply whole genome sequencing technology – that is also called massively parallel sequencing, because it can sequence different bits of genomes at the same time in parallel, we can derive multiple species barcodes from a single sample. This is called metabarcoding. This may be familiar to those with a penchant for eDNA (environmental DNA) studies, as we can apply it to total DNA extracted from environmental samples, as well as pooled bits of biological tissue.
However, to do any barcoding (singular or meta) we must first be sure that our target species (e.g., mosquitoes) can be differentiated with barcoding, and with an appropriate barcode region of the genome. This is exactly what Villeneuve and colleagues did in 2024 on our foci of A. impiger and A. nigripes. This study collected samples from each species from four sites across the North American Arctic, including Toolik Alaska, Cambridge Bay and Karrak lake Nunavut, and Kuujjuaq, Nunavik, northern Quebec. Females of the species were morphologically identified and subject to DNA extraction. They were all them barcoded at two regions: COI and ITSR2 (internal transcribed spacer region 2). COI barcoding confirmed that A. impiger and A. nigripes could be differentiated on the basis of genetic alone; however, the ITSR2 locus failed to resolve the two species, underscoring how barcode regions need to be tested for veracity. COI can now be used to monitor, at scale in the Arctic, for the presence of range shifts in response to climate change, habitat alteration, or incursion and competition with other species (competitors or predators) or A. impiger and A. nigripes. Indeed, COI barcodes have been screened for numerous Canadian species allowing for the full diversity of Culicidae to be tracked in the future.
What about tracking pathogens and disease? Very recent work has found the presence of illness-causing Jamestown Canyon Virus in our focal species in the Canadian Arctic, albeit as yet not a fatal ailment. Can we use genomics methods to monitor and study the communities of potential pathogens that mosquitoes may be more susceptible to in a changing Arctic? In a word: yes. Last year, a study of our two foci species used whole genome sequencing to sequence the total RNA extracted from each species. RNA sequencing can not only sequence the products of genes of the parent organism, but also the genes of pathogens like viruses, especially if they have RNA (not DNA) genomes (some viruses have RNA genomes, some have DNA genomes). This study found that the diversity of viral genomes contained within each species was relatively unique and included viral genomes hitherto unknown to science. These findings suggest that each species has a unique interaction with a different suite of viral particles that they may vector to other animals in the High Arctic, and that a divergent array of viral families are represented and replicate within the mosquitoes, at least in Greenland where samples were collected. These data are new, and more work needs to be done to test the influence of location and intrapopulation variability on the viral load of mosquitoes, along with other possible pathogens; and whether the risk of zoonotic transmission to mammals (including humans) is influenced by a warming Arctic.
© Arctic Institute of North America, University of Calgary
Site & Image Information